
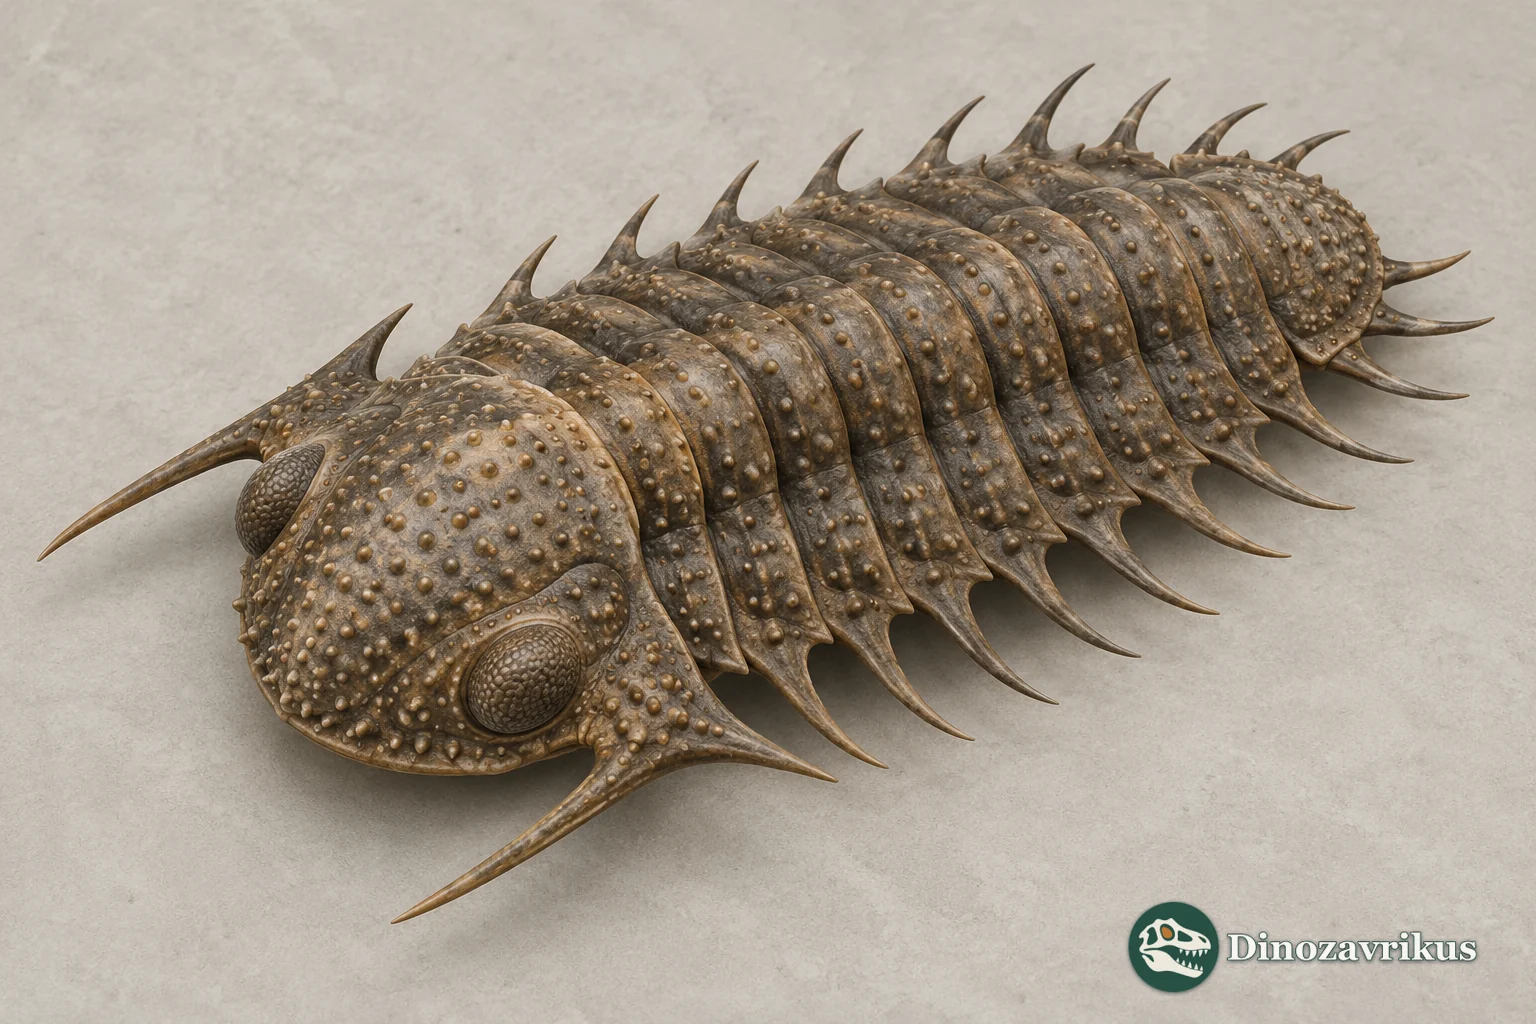
Leonaspis is a genus of odontopleurid trilobites with a tuberculate shell and numerous marginal spines. Its type species, Leonaspis leonhardi, comes from Ludlow-age strata in Bohemia. The spiny outline is conspicuous, but classification depends on a combination of cephalic, thoracic and pygidial characters rather than one dramatic tail feature.
During the twentieth century, many spiny species from different regions were grouped in Leonaspis. A phylogenetic revision found that this broad genus was polyphyletic. A 2024 study further emphasised spine variability and growth. Older reports of its age and geography therefore need to be read in light of the diagnosis used by each author. The genus is included in the ancient arthropod catalogue as an example of how morphological revision changes a genus boundary.
Quick facts
| Scientific name | Leonaspis Richter & Richter, 1917 |
|---|---|
| Type species | Leonaspis leonhardi (Barrande, 1846) |
| Group | Trilobita, Odontopleurida, Odontopleuridae |
| Type interval | Ludlow, Late Silurian |
| Type region | Kopanina Formation, Barrandia, present-day Czechia |
| Classic narrow diagnosis | Nine thoracic segments plus a suite of pygidial characters |
| Observed variation | L. leonhardi specimens have two to five interior marginal spines |
| Evidence limit | Isolated shields may not preserve enough characters for a secure genus assignment |
What can the fossils tell us?
The type species is Odontopleura leonhardi Barrande, 1846, from the Ludlow Kopanina Formation in Barrandia. A type species anchors the name Leonaspis; it does not automatically place every similar spiny fossil in the genus.
The classic narrow diagnosis uses nine thoracic segments, their proportions and a combination of cephalic and pygidial characters. Disarticulated shields often do not preserve the full combination.
Specimens of the type species show two to five interior marginal spines. The 2024 study relates some differences to development and documents variability, so spine count must be assessed with other characters.
The 1991 phylogenetic revision divided the older polyphyletic concept and moved species to Kettneraspis and Exallaspis. Later work revisited segmentation and species assignments, so distant records are not automatically a confirmed range for one genus.
Name and taxonomic history
Rudolf and Emma Richter established Leonaspis in 1917. By original designation, its type species is Odontopleura leonhardi, described by Joachim Barrande in 1846; the species is now usually cited as Leonaspis leonhardi. Its type region is Barrandia, a historically important fossil district in Central Europe, and the type beds are Ludlow in age.
The genus was first applied broadly to many spiny forms. In 1991, Lars Ramsköld and Brian Chatterton tested the characters in a phylogenetic framework and concluded that this broad assemblage included separate lineages. Their narrower Leonaspis concept combined nine thoracic segments with usually four interior pygidial border spines; other species were reassigned, including to Kettneraspis and Exallaspis.
That revision was important, but it did not end discussion. In 2024, van Viersen reassessed postcephalic segmentation and spines in Silurian–Devonian odontopleurines. The type species L. leonhardi shows more variation than a simple “four versus two” rule allows. Interior spine number changes during development and varies among specimens, so additional characters remain necessary.
Cephalon, thorax and pygidium
The cephalon was broad and vaulted. Tubercules covered the central glabella and cheek regions, and long genal spines projected from the rear corners. Their proportions and surface pattern varied among species, although the armoured outline is characteristic of the family.
The classic diagnosis of narrow Leonaspis counts nine thoracic segments. Their proportions and armature help distinguish it from related genera. Some anterior segments are shorter than those farther back, and the pleural portions carry lateral spines. An articulated fossil is especially useful because it connects the cephalic, thoracic and pygidial features used in classification.
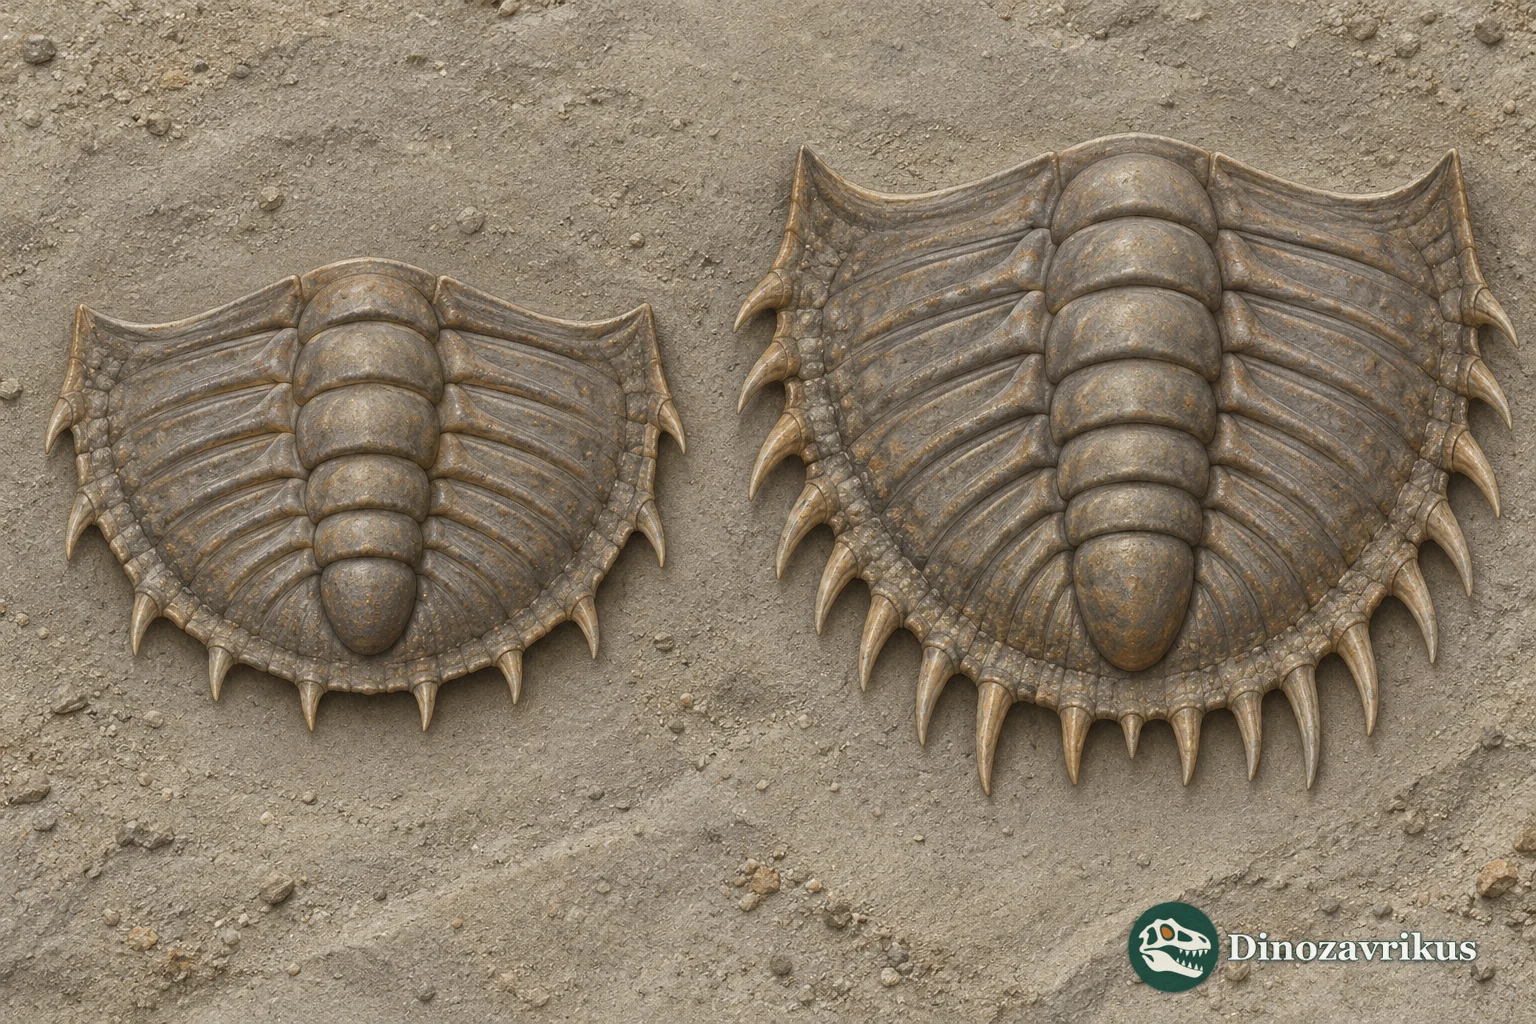
The pygidium is the tail shield formed by fused posterior segments. Several pairs of spines fringe its margin, while interior border spines have been used to distinguish genera. Specimens of L. leonhardi have been described with two, three, four or five interior spines. Growth and individual variation complicate the count, so a fragmentary pygidium alone cannot replace a full morphological comparison.
Growth and spine variation
Trilobites grew by moulting and shedding the outer shell. Juveniles differed in the proportions of the head and tail shield, and some spines or tubercles became more developed as segments formed. Comparing pygidia of different sizes without an ontogenetic series can be misleading: juvenile and adult forms may look like separate taxa, while adults in one species may differ in the number of marginal elements.
Variation can have more than one cause. Some differences follow growth; others may be individual anomalies or the result of injury and repair. A taxonomic diagnosis therefore benefits from a series of specimens, comparable parts of the pygidium and thoracic segmentation where available. This is why spine number is treated as useful evidence rather than a single decisive test.
Fossil shells often break into separate shields. Moulting, decay, movement across the seafloor and currents can disarticulate a body before burial. Compaction may hide a small spine or make a crack look like a segment boundary. Articulated fossils and carefully prepared specimens provide stronger evidence, but are less common than isolated pieces.
Age, fossil material and geography
The type species comes from the Ludlow-age Kopanina Formation in Barrandia. Other species assigned after revisions come from Silurian and Devonian rocks in several regions. A compiled database may show a broader span, including the Middle Ordovician, but the earliest and most distant assignments reflect broader historical concepts and require review.
Species described from Central Europe and the British Isles contribute to the Silurian record; Devonian odontopleurines have also been studied in Morocco, Australia and North America. These reports should not be combined into a single confirmed range for Leonaspis. Some material has moved to other genera, and some newer European records remain tentative because of similarities with Kettneraspis.
The strength of a record depends on what was found. An isolated cheek or tail shield may confirm an odontopleurid, but not necessarily Leonaspis. Articulated specimens, thoracic segment counts and a consistent set of characters provide a stronger basis. Age limits should therefore be tied to specific species descriptions, not only to an aggregated database entry.
Habitat, spines and limits of inference
Leonaspis lived in marine settings and moved along the seafloor. The sediment and associated fauna help reconstruct conditions at a particular locality, but the genus did not necessarily occupy one uniform substrate everywhere. Soft appendages are not normally preserved in the material used to identify it; details of locomotion are inferred from other trilobites.
The function of the spines remains a hypothesis. They increased the apparent body outline and may have made capture more difficult; their shape may also have affected contact with the substrate. The shell does not prove that a particular pair served defence, stabilisation or display. Organisms found colonising odontopleurid spines record post-mortem occupation and preservation, not direct behaviour by the living trilobite.
Diet is also unknown. Eyes and a benthic setting are consistent with activity near the bottom, but cannot distinguish deposit feeding, scavenging or another feeding mode. No gut contents establish the diet of Leonaspis.
When did the type species of Leonaspis live?
Leonaspis leonhardi comes from the Ludlow, Late Silurian, in the Kopanina Formation of Barrandia. Other species assigned to the genus have Devonian records, but not every older identification meets the current diagnosis.
Did every Leonaspis have four interior tail spines?
No. Specimens of the type species have been described with two to five interior marginal spines. Counts vary with growth and among specimens, so they are considered alongside thoracic and other pygidial characters.
How is Leonaspis distinguished from Kettneraspis?
Researchers compare a combination of cephalic, thoracic and pygidial features. A spine count alone is unreliable for an isolated specimen, especially when its growth stage is unknown.
What were the spines used for?
Defence or an effect on posture near the seafloor are possible, but direct behaviour is not preserved. Fossils show shell shape, not the animal's use of each spine.