
Lonchodomas is an Ordovician genus of blind raphiophorid trilobites distinguished by a glabella that projects forward into a long rostral spine. Its short thorax and rear parts are known mainly from separate fossil shields. New work on one species, L. chaziensis, has added a detailed record of juvenile growth, while the spine's function remains uncertain. The ancient arthropod catalogue sets Lonchodomas beside other trilobites with different head shapes and ecological evidence.
Quick facts
| Scientific name | Lonchodomas Angelin, 1854 |
|---|---|
| Type species | Ampyx rostratus Sars, 1835 |
| Group | Arthropoda, Trilobita, Raphiophoridae |
| Age | Ordovician; species records span regional intervals |
| Diagnostic feature | Glabella extends forward into a long rostrum |
| Thorax | Typically five articulating segments |
| Known material | Mostly separate cranidia, thoracic parts and pygidia |
| Diet and size | No direct diet evidence or genus-wide length |
What can the fossils tell us?
Sars described Ampyx rostratus in 1835; Angelin established Lonchodomas in 1854. Later workers used the species as the type of the genus. Its name-bearing role is distinct from the many species and partial specimens subsequently assigned to Lonchodomas.
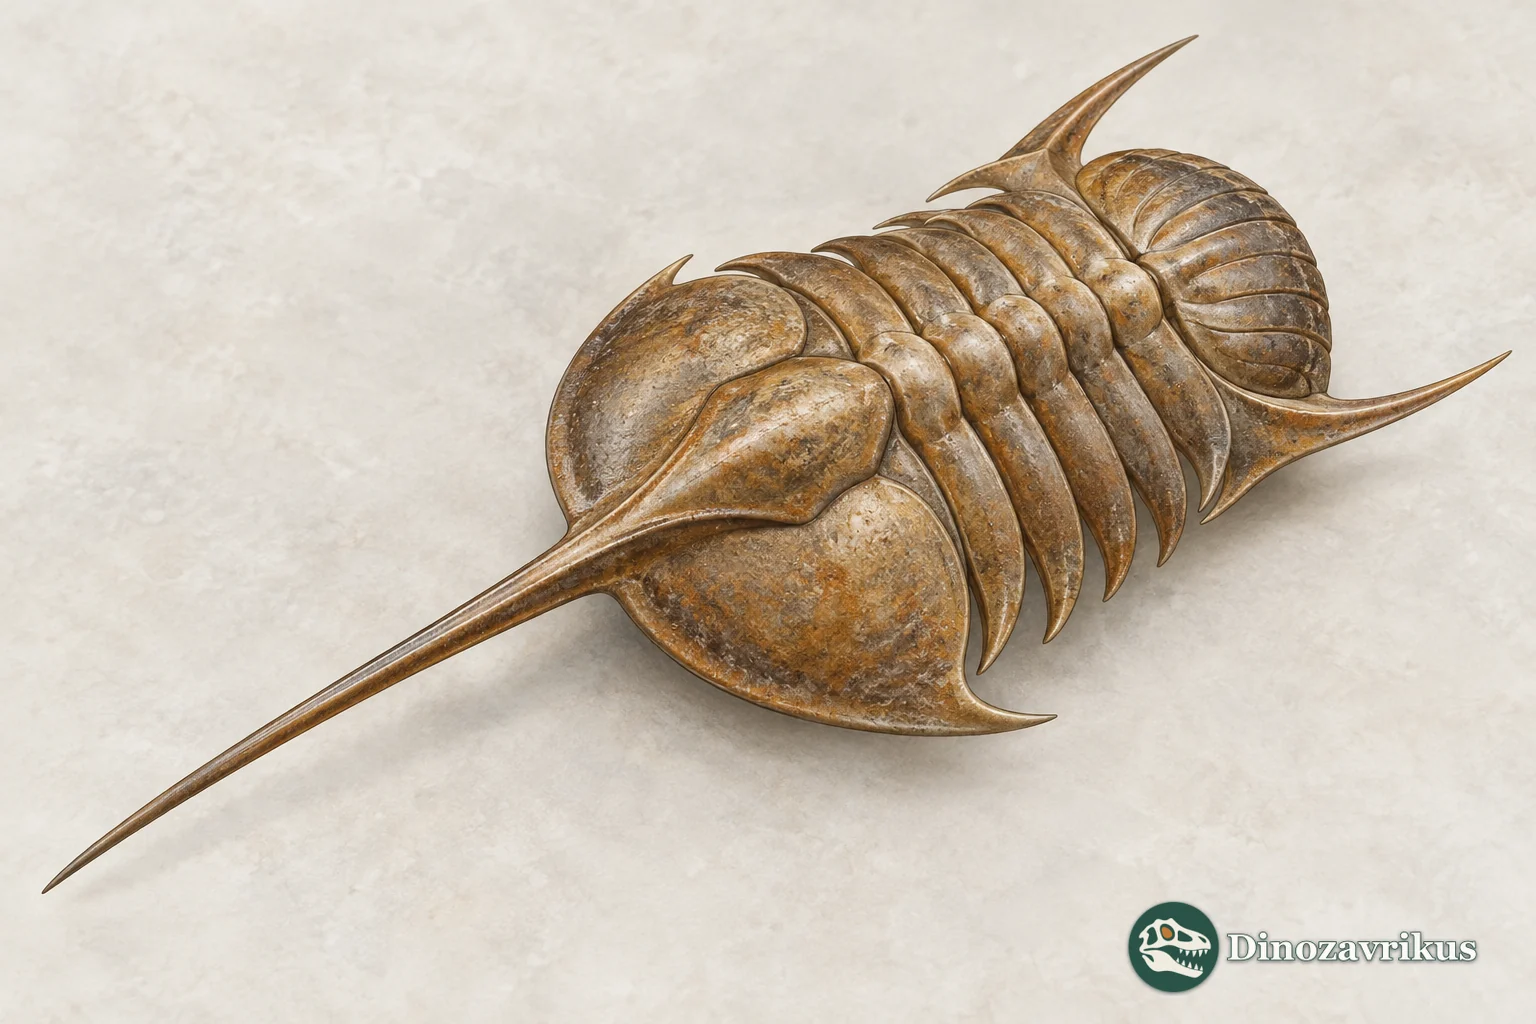
Typical forms have a forward-extended, often ridged glabella, a short thorax of about five segments and a small transverse pygidium. Developed eyes are not known. The shell does not reveal the spine's purpose.
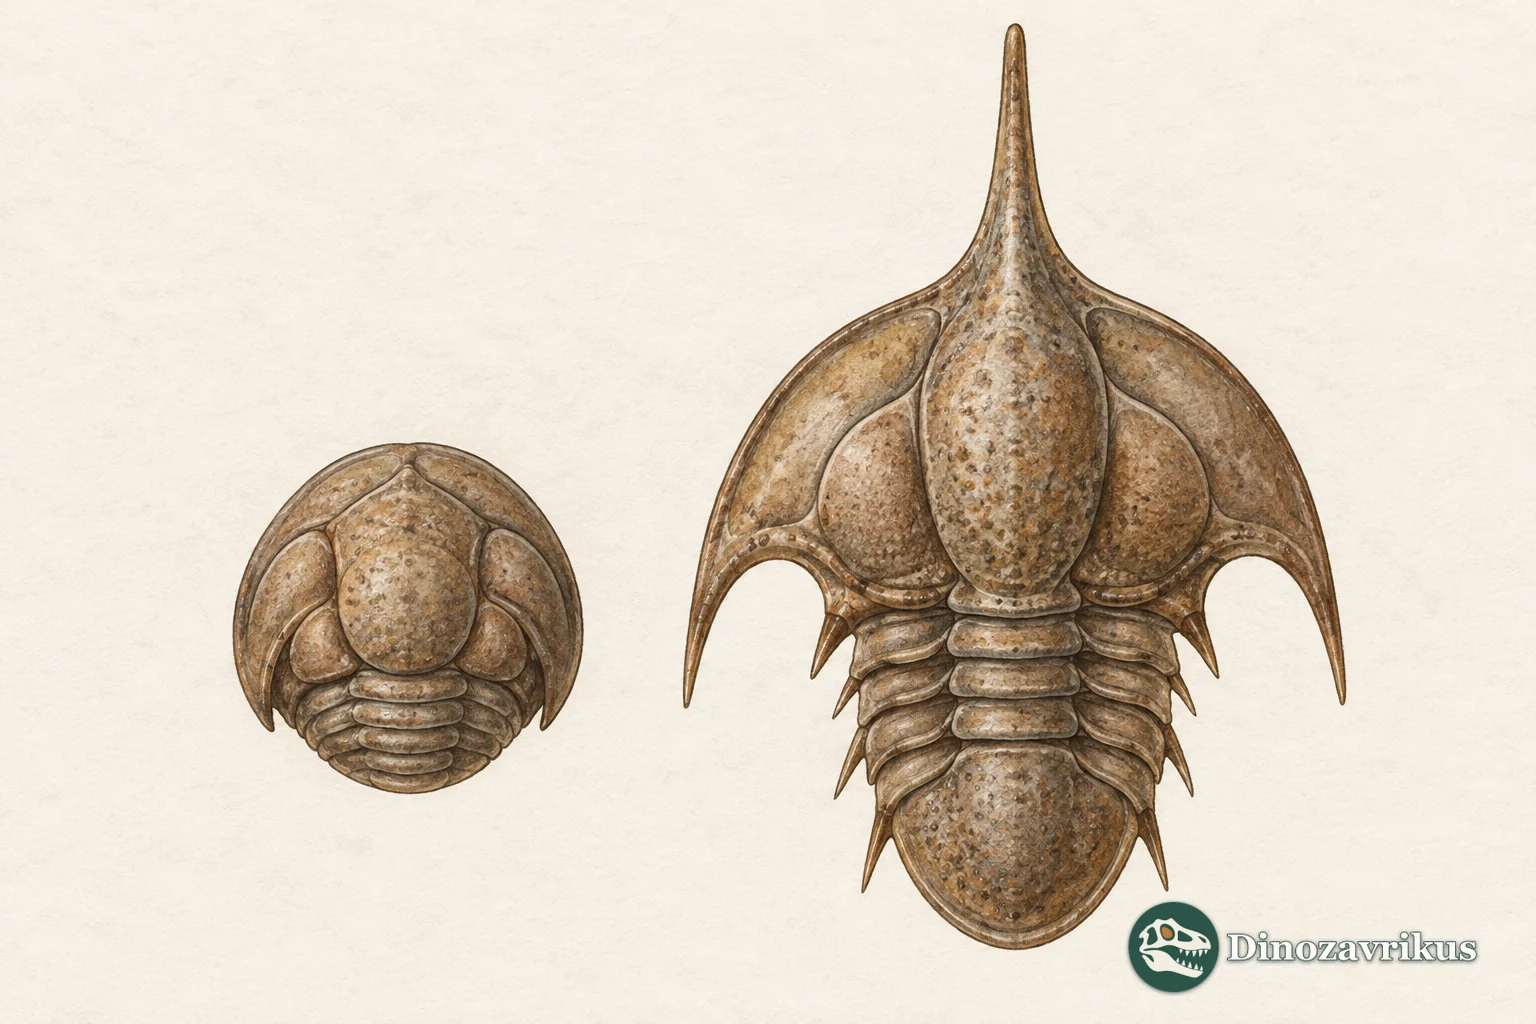
A 2026 study compared three successive instars of Lonchodomas chaziensis from one thin horizon in New York. Head shape and modular organisation changed sharply between a later protaspid and the first meraspid stage. This is evidence from one species and sample.
Defence, support, sensing and sexual selection have been proposed for long raphiophorid spines. They remain hypotheses for Lonchodomas; no direct feeding trace or behavioural fossil settles the question.
A name tied to Ampyx rostratus
Nils Peter Angelin established Lonchodomas in 1854. The type species is Ampyx rostratus, described by Michael Sars in 1835 and later transferred to the genus. The type fixes how the name is used, but it does not represent every form later placed in Lonchodomas.
The genus belongs to Raphiophoridae, a family of trilobites with blind cranidia and striking spines. A later spelling, Lonchodomus, appears in older nomenclatural records, but it is not treated as a separate accepted genus. Species diagnosis relies on combinations of glabellar shape, facial sutures, rear head spines and pygidial proportions.
The long rostrum and compact trunk
In typical forms, the convex glabella narrows toward the front and continues into a straight, solid rostrum. A median crest may run back from the spine. Paired spines extend from the rear corners of the head shield. The thorax is short, commonly with five articulating segments, and the pygidium is relatively small and transverse.
Developed compound eyes have not been described for the genus. Blindness is consistent with reduced light or close contact with the substrate, but it does not identify a precise depth. Soft limbs are rarely preserved, so reconstructions borrow cautiously from related trilobites.
A dramatic juvenile transition in one species
In 2026 Ernesto Vargas-Parra and Melanie Hopkins examined three successive instars of Lonchodomas chaziensis from the Middle Ordovician Crown Point Formation on Valcour Island, New York. To limit time averaging, they collected material from one horizon only about two centimetres thick near Pebble Beach. Buffered formic acid processing yielded silicified, mostly disarticulated sclerites, so the study concentrated on the head.
The sample included two protaspid stages and the first meraspid stage. Between the later protaspid and meraspid instar, the head changed markedly in outline and in the way anatomical regions covaried. The authors' modularity analysis supported a shift from three modules to two. This is a statistical description of shape relationships, not a count of body parts.
The authors discuss a possible shift from a planktonic early stage to a more benthic juvenile. The sequence itself is fossil evidence; the exact movement and habitat transition are inferred. The result belongs to L. chaziensis and should not be assumed for all species of Lonchodomas.
What might the spine have done?
Protection, stabilisation on soft sediment and a sensory role have all been proposed for long trilobite spines. A 2005 comparison of raphiophorid spines with beetle horns noted that relative spine length could change through growth and that close relatives sometimes differed strongly in shape. The authors suggested sexual selection or competition as possibilities.
That study did not demonstrate courtship or combat in Lonchodomas. No soft sensory structures are preserved at the tip, and the fossil record does not show the spine in use. Several functions could also have acted together. The similar rostrum of Ampyx offers a comparison of anatomy, not proof of identical behaviour.
Ordovician range and ecological limits
Named and open-nomenclature material attributed to Lonchodomas has been reported from Lower through Upper Ordovician rocks in North and South America, Europe and Asia. The type species is known from Scandinavia. This broad range combines different species and regional successions rather than tracking one continuous population.
Many fossils are isolated cranidia or pygidia. Even when pieces carry the same genus name, they may come from separate beds or localities and cannot automatically be assembled into one animal. The age of each find comes from the enclosing rock and its associated fossils.
Trilobites moved with jointed limbs and grew through moults, but no direct gut content or trace establishes the diet of Lonchodomas. The blind head and compact trunk are compatible with benthic adults, while the new juvenile series raises the possibility of different early habitat use in one species. Neither shell shape nor the long rostrum gives a reliable body length, swimming speed or feeding method. Asaphus, with its very different eye arrangements, illustrates how varied Ordovician trilobite sensory anatomy could be.
Frequently asked questions
When did Lonchodomas live?
The genus is known from Ordovician rocks. Individual species have separate regional age ranges.
What was the long spine for?
Its function is unknown. Protection, stabilisation, sensing and sexual selection have been proposed, but none is demonstrated directly for the genus.
What is known about Lonchodomas growth?
A 2026 study documented a sharp change across one moult in Lonchodomas chaziensis. It examined one species and a tightly sampled horizon.
What did Lonchodomas eat?
No direct feeding trace is known. A benthic diet is possible but cannot be specified from the shell alone.