
Panorpidium is an extinct genus of elcanid orthopterans, an early branch of the grasshopper-and-cricket order rather than a member of any living family of grasshoppers. Its best-known features are the branching veins of the forewing and long, jointed spurs on the hind tibia. Most well-supported records are Cretaceous, but a single Tithonian wing from Poland was assigned to ?Panorpidium polonicum in 2026, provisionally extending the genus into the Late Jurassic. Those traits are not preserved together in every fossil: the name itself is anchored by an isolated wing, while later Asian specimens reveal more of the insect.
Fossil impressions from Europe and Asia record wings and, in some cases, legs or bodies. Mid-Cretaceous amber from Myanmar preserves particularly fine details, while a 2026 revision of 88 Brazilian Crato specimens transferred Cratoelcana damianii to Panorpidium. Researchers still disagree about whether one amber species belongs in Panorpidium or a separate genus.
Quick facts
| Scientific name | Panorpidium Westwood, 1854 |
|---|---|
| Type species | P. tessellatum Westwood, 1854 |
| Family | Elcanidae, order Orthoptera |
| Known interval | Late Jurassic? to Cretaceous; oldest referral is tentative |
| Type material | A forewing from Durlston Bay, England |
| Key characters | Wing venation and jointed hind-tibial spurs |
| New combination | Panorpidium damianii from the Crato Formation |
What can the fossils tell us?
The type does not preserve the head, mouthparts, antennae or hind legs. Details of the body come from other species assigned to the genus.
Its venation supports a provisional assignment to Panorpidium. The question mark reflects uncertainty; it is not a settled oldest occurrence.
Carbon mapping helped reveal branching in Korean P. spica, but analytical imaging cannot restore missing anatomy.
A water-surface function was proposed for broad lobes in P. spica. No fossil records the behaviour, and the hypothesis does not apply automatically to all species.
A genus founded on one wing
John Obadiah Westwood named Panorpidium tessellatum in 1854 from a forewing collected at Durlston Bay, Dorset, in southern England. The type specimen is held by the Natural History Museum, London. Its original geological label referred to the Middle Purbeck beds; modern stratigraphy places the relevant Purbeck succession in the upper Berriasian, near the beginning of the Cretaceous.
A wing-only type fixes what the genus name means through the shape and venation of that wing. It cannot directly tell us what the insect’s head, mouthparts, antennae or hind legs looked like. Those body features come from other named species that researchers compare with Westwood’s type. Some older classifications also brought names such as Elcana and Baisselcana into synonymy with Panorpidium. Because the evidence and taxonomic concepts changed over time, a broad range assembled from every historical combination should not be treated as a single secure lineage.
The better-supported records include Early Cretaceous material from England and Asia, as well as younger amber specimens. This is a useful distinction between the age of the oldest type record and the range of species later assigned to the genus. Not every occurrence is equally diagnostic, especially when only part of a wing is preserved.
Reading a fossil wing
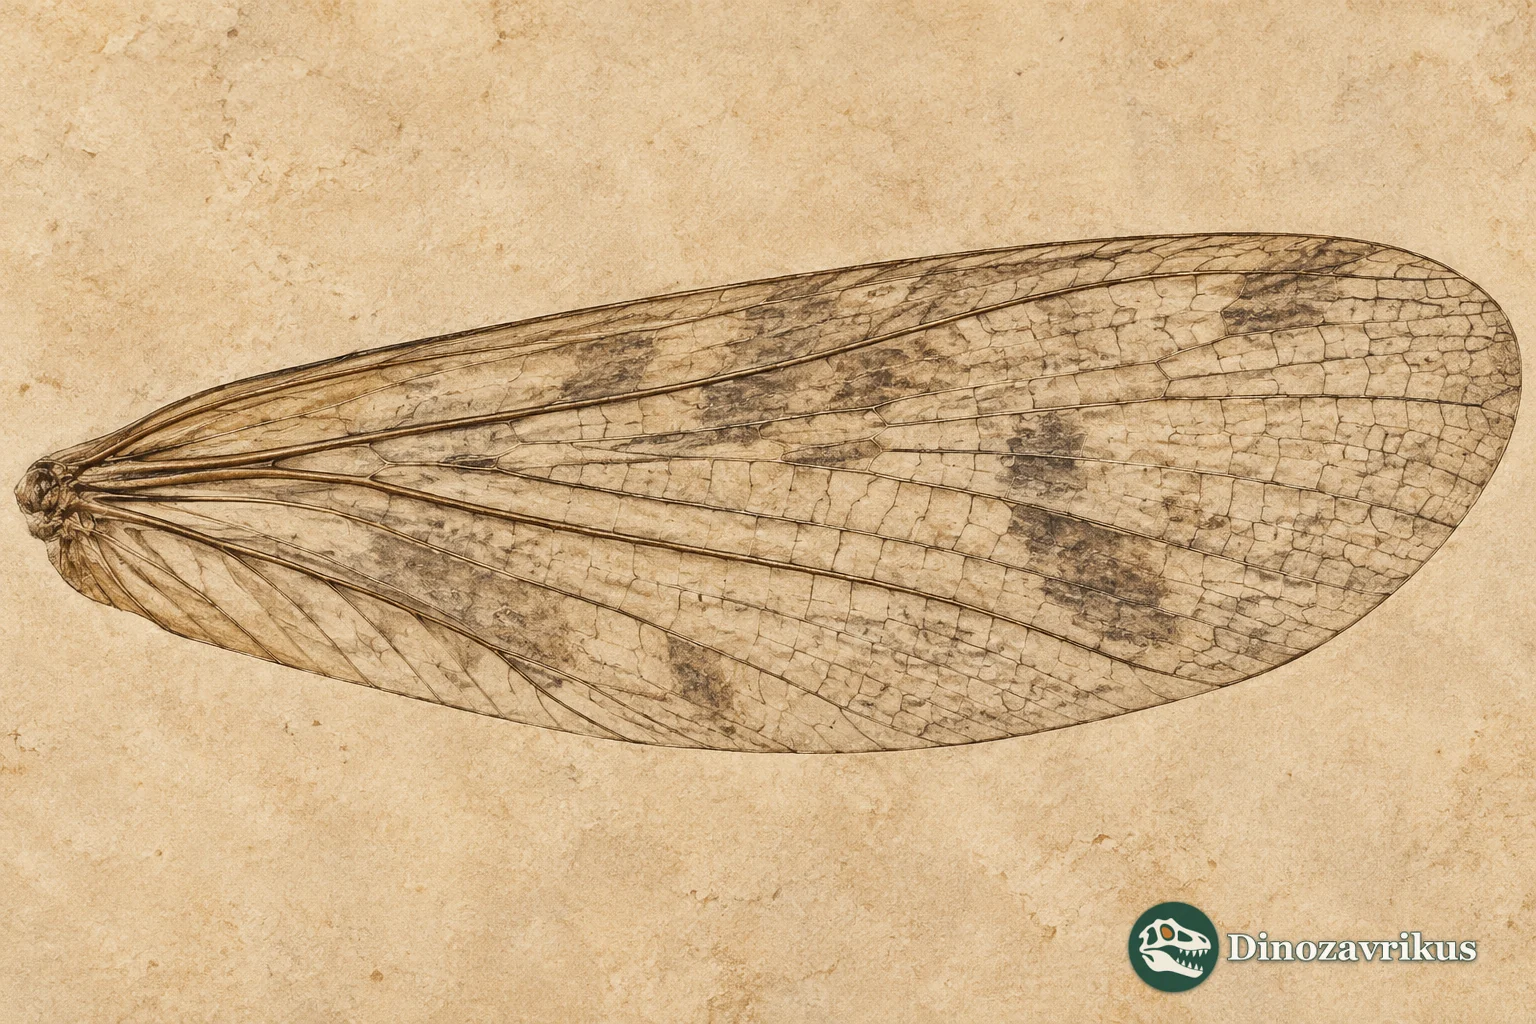
The forewing, or tegmen, was relatively narrow and more leathery than the hind wing. Palaeoentomologists compare the paths and branching patterns of the posterior subcosta (ScP), anterior and posterior radius (RA and RP), media (M), and cubital veins. They also inspect cross-veins, the width of wing fields and any preserved dark patches. This network acts as a set of anatomical characters when the fossil contains no complete skeleton.
A specimen from the Yixian Formation in China, assigned to P. yixianensis, preserves parts of the thorax, three right legs and wings. Its holotype, NIGP 159068, has a forewing 23.4 millimetres long. The associated hind tibia measures 12.9 millimetres, and its longest spur approaches 4 millimetres. These are measurements of one species and individual, not a standard size for the genus. The dark rounded patch on this wing is also not evidence that the English type species had the same marking.
Three specimens of the Korean species P. spica come from the lower Albian Jinju Formation. Some veins were difficult to see in ordinary photographs. Researchers used wavelength-dispersive spectrometry to map carbon concentrations, making parts of the RA and RP branching and some abdominal structures clearer. This method reveals chemical contrasts already present in the fossil; it does not restore missing anatomy or turn an uncertain outline into a complete insect.
A tentative Late Jurassic occurrence
In 2026, Monika Michalska and Błażej Błażejowski described ?Panorpidium polonicum from a single nearly complete right tegmen in the Tithonian Kcynia Formation at Owadów-Brzezinki, central Poland. The preserved imprint is about 25 mm long; the authors estimate an original length near 29 mm. Venation supports a provisional placement in Panorpidium, but the question mark matters: this is a possible older record, not an uncontested extension of the genus.
Hind legs and movable spurs
Elcanids had enlarged hind femora that housed the muscles used for jumping. Their tibiae carried pairs of long spurs attached by joints, rather than fixed projections fused to the leg. The shape differs across species: some spurs are slender and spine-like, while others broaden into leaf-shaped lobes. Additional spurs occur near the tibial tip, and short, stout spines may line the underside of the first hind-tarsal segment.
In P. spica, the broad tibial lobes were compared with structures in living pygmy mole crickets (Tridactylidae). The authors proposed that they might help the insect jump from a water surface or submerge briefly to escape. A pterostigma on the wing also informed a hypothesis of short, controlled flights. These are functional interpretations based on shape and comparison, not behaviours recorded by a trace fossil. The researchers did not exclude other uses for the spurs, and a water-surface function cannot be extended automatically to species with narrow spines.
Amber reveals the body, but not consensus
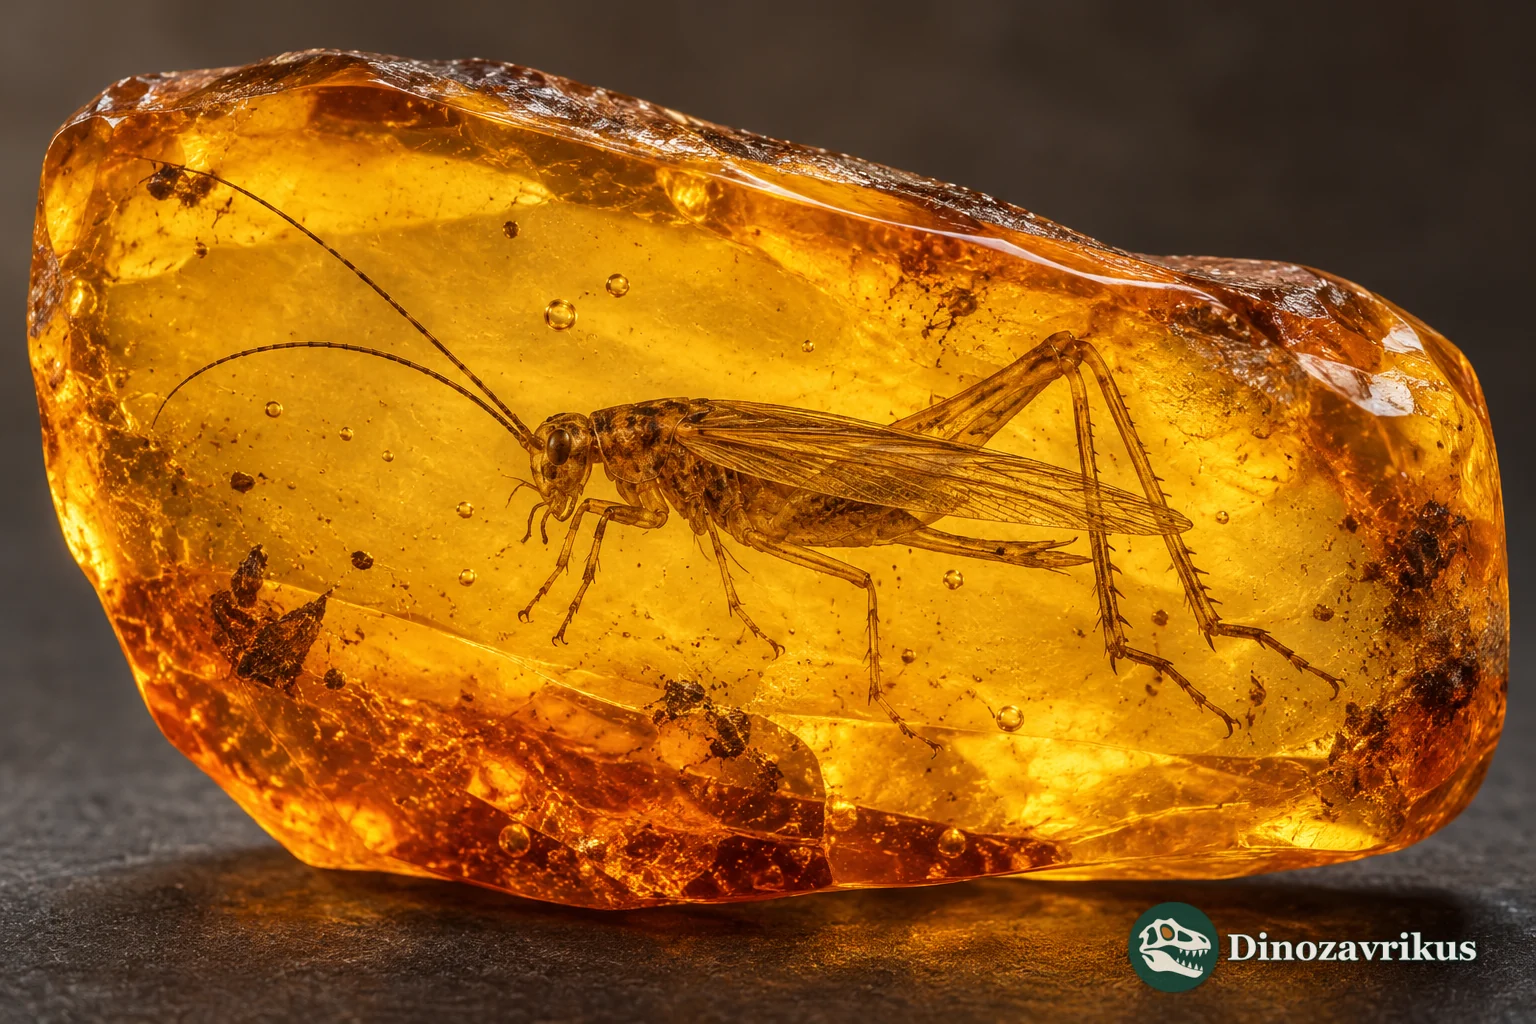
Myanmar amber from the mid-Cretaceous preserves more than a flattened wing. Specimen YU-OR-100001, described in 2022 as Panorpidium maculosum, retains antennae, legs and wings. Its ScP vein divides into six branches. Paired spine-like spurs occur along the posterior half of the hind tibia, three more stand at its tip, and a row of robust spines runs beneath the first segment of the hind tarsus. The combination of venation and legs led researchers to unite the earlier amber genus Burmelcana with Panorpidium.
That interpretation remains contested. A 2025 study placed P. maculosum in a new genus, Pseudopanorpidium, emphasizing proportions near the rear margin of the tegmen and other differences. A separate 2025 paper retained the species in Panorpidium and described P. stenos as another Myanmar species. The disagreement concerns which characters define the genus, not whether the amber fossils preserve real wings and legs. Until authors agree on the diagnosis, it is clearer to name the competing treatments than to present one as settled.
The Crato Formation revision
A 2026 study examined 88 elcanid specimens from Brazil’s Lower Cretaceous Crato Formation. It transferred Cratoelcana damianii to Panorpidium as P. damianii and moved C. rasnitsini into the new genus Mesembrelcana, leaving Cratoelcana monotypic. The authors also discussed why females make up 69.3% of their sample, including possible sex-biased preservation or a stronger association with aquatic egg-laying habitat. These are hypotheses about the assemblage, not direct observations of behaviour.
What behaviour can be inferred?
A strong jumping leg and two pairs of wings support the conclusion that adult elcanids could jump and fly. Long antennae probably had a sensory role, as they do in many insects, but that is an inference from comparative anatomy. The type species’ mouthparts are unknown, and no gut contents, eggs or egg-laying structures are securely associated with Panorpidium. Its diet might have been plant-based, mixed or something else; the fossils do not decide among those possibilities.
The possible Late Jurassic occurrence in Poland would extend the known history of the genus if the provisional identification is confirmed. For now, that conclusion depends on one wing and a cautious taxonomic interpretation. Colour, antenna posture, vegetation and the insect’s stance in an illustration remain artistic choices. The fossils provide the clearest evidence where they preserve vein networks, jointed spurs and, in amber, body outlines.
Frequently asked questions
When did Panorpidium live?
Most well-supported species are Cretaceous, from upper Berriasian beds in England to mid-Cretaceous deposits in Asia and Brazil. A Tithonian Polish wing was assigned provisionally as ?Panorpidium polonicum in 2026.
What were the hind-leg spurs for?
The spurs were jointed parts of the hind tibia, on legs adapted for jumping. Broad lobes in P. spica inspired a hypothesis about moving or jumping across water, but that function is not directly demonstrated and may not apply to every species.
What is known about the type species?
Panorpidium tessellatum is based on a single forewing from Durlston Bay, England. Its outline and venation are directly known, whereas the head, mouthparts, antennae and hind legs are not represented by the type.
Why is the genus classification disputed?
Researchers differ over whether the Myanmar amber species P. maculosum has the wing proportions of Panorpidium or should be placed in Pseudopanorpidium. Recent papers have adopted both treatments.