
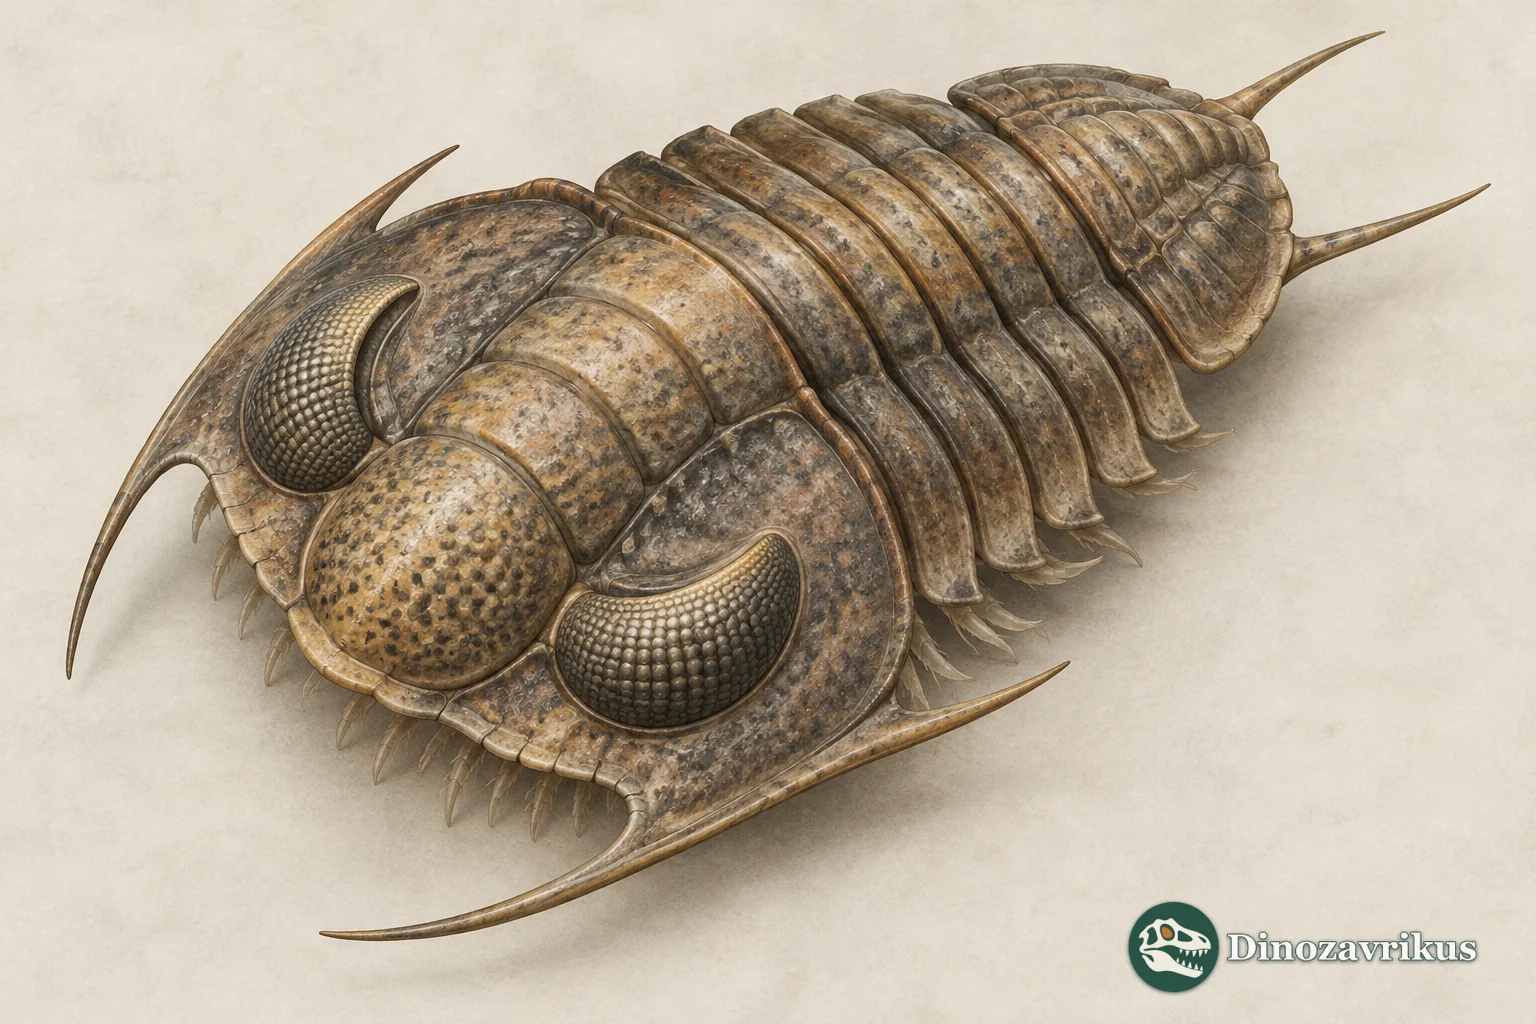
Telephina is an Ordovician genus of small trilobites in the family Telephinidae. Large compound eyes and, in some species, slender spines distinguish its fossils. Together with their distribution, these traits support a life in the water column, though no fossil records a particular swimming speed or depth. The ancient arthropod catalogue places Telephina among trilobites with very different eyes, shells and inferred habitats.
Quick facts
| Scientific name | Telephina Marek, 1952 |
|---|---|
| Type species | Telephus fractus Barrande, 1852 |
| Group | Arthropoda, Trilobita, Telephinidae |
| Age | Ordovician; ranges vary among species |
| Type record | Králův Dvůr Formation, Bohemia |
| Known material | Cranidia, eyes, thoracic segments and pygidia |
| Likely ecology | Pelagic or near-pelagic, inferred from several traits |
| Size and diet | No genus-wide length or direct diet evidence |
What can the fossils tell us?
Ladislav Marek established Telephina in 1952 with Telephus fractus Barrande, 1852 as its type species. The species comes from the Upper Ordovician Králův Dvůr Formation. Telephina replaced the preoccupied name Telephus; the two names do not represent separate animals.
Fossils show the cranidium, eye surfaces and, in some species, slender spines. The features vary among species and growth stages. They do not preserve exact vision, soft limbs or colour.
Chatterton, Edgecombe, Vaccari and Waisfeld documented a marked late meraspid transition in Telephina calandria, T. chingolo and T. problematica. The finding applies to those species and samples, not automatically to the whole genus.
Large eyes, shell proportions, spines and geographic occurrence support a pelagic or near-pelagic interpretation. They do not establish swimming speed, depth or continuous separation from the seabed.
A replacement name with a Bohemian type species
Ladislav Marek established Telephina in 1952 and designated Telephus fractus, described by Joachim Barrande in 1852, as its type species. Nikolaisen's 1963 revision identifies the type locality with the Upper Ordovician Králův Dvůr Formation of Bohemia. The genus name Telephus was already occupied, so Telephina is a replacement name rather than a second genus based on a different fossil.
Species from Norway, Sweden, Estonia, Argentina, North America and other regions have since been assigned to the genus. Nikolaisen grouped some forms with paired frontal glabellar spines in a subgenus, Telephina (Telephops). Later authors differed over whether those spines justify a separate subgenus, in part because related structures can change during growth. Taxonomic comparisons therefore use the whole cranidium, facial sutures, eye lobes and pygidium instead of one conspicuous feature.
Large eyes and a variable shell
The head shield, or cranidium, carries broad compound eyes formed from many small lenses. Their size is directly visible, but exact visual acuity, colour discrimination and behaviour are not. Some species also have long genal or posterior spines; others are distinguished by paired structures on the front of the glabella. A genus-level illustration should not imply that every named species shared the same spines.
Telephinid remains are commonly disarticulated. A cranidium, a free cheek, a thoracic segment and a pygidium may be collected separately, so the complete animal is assembled by comparison rather than found as one articulated individual. The soft limbs and the lower side of the body are less securely known.
Occurrences from Bohemia to Estonia
The type species comes from the Upper Ordovician of Bohemia, while other species range through several Ordovician intervals. In 2010 Helje Pärnaste found a cranidium assigned to Telephina (Telephops) biseriata in a loose boulder from the Sompa mine tip-heap near Kohtla-Järve, northeastern Estonia. Adrian Popp donated it to the Institute of Geology at Tallinn University of Technology, where it is catalogued as GIT 360-335.
The specimen came from kerogenous limestone of the Viivikonna Formation and Kukruse Regional Stage, dated to the Sandbian. Because it was collected from a mine tip-heap rather than a measured bed, the exact position in the original section is unknown. It provides a first published Estonian record of the genus, not a direct measure of how common it was across the region.
Other Scandinavian records occur in named formations and biozones. Those stratigraphic contexts help correlate separate marine sequences, but a genus-level map combines species that lived at different times and in different settings.
Why researchers infer a pelagic habit
Large eyes, a compact shell, spines and occurrences in more open-water faunas make a pelagic or near-pelagic ecology plausible. Bruton and Høyberget reconstructed Telephina bicuspis from the Middle Ordovician Oslo region as a pelagic trilobite. Pärnaste and Popp discussed the Estonian occurrence alongside other genera known from deeper-water settings, while also noting the local stratigraphic context.
These are ecological interpretations from several lines of evidence. A shell by itself cannot tell whether an animal swam constantly, rose into the water column at certain times, or was moved after death. Large eyes also occur in trilobites with other habits, so they are not decisive alone. The blind Ordovician trilobite Ampyx offers a useful contrast in sensory anatomy.
Growth changed the body plan
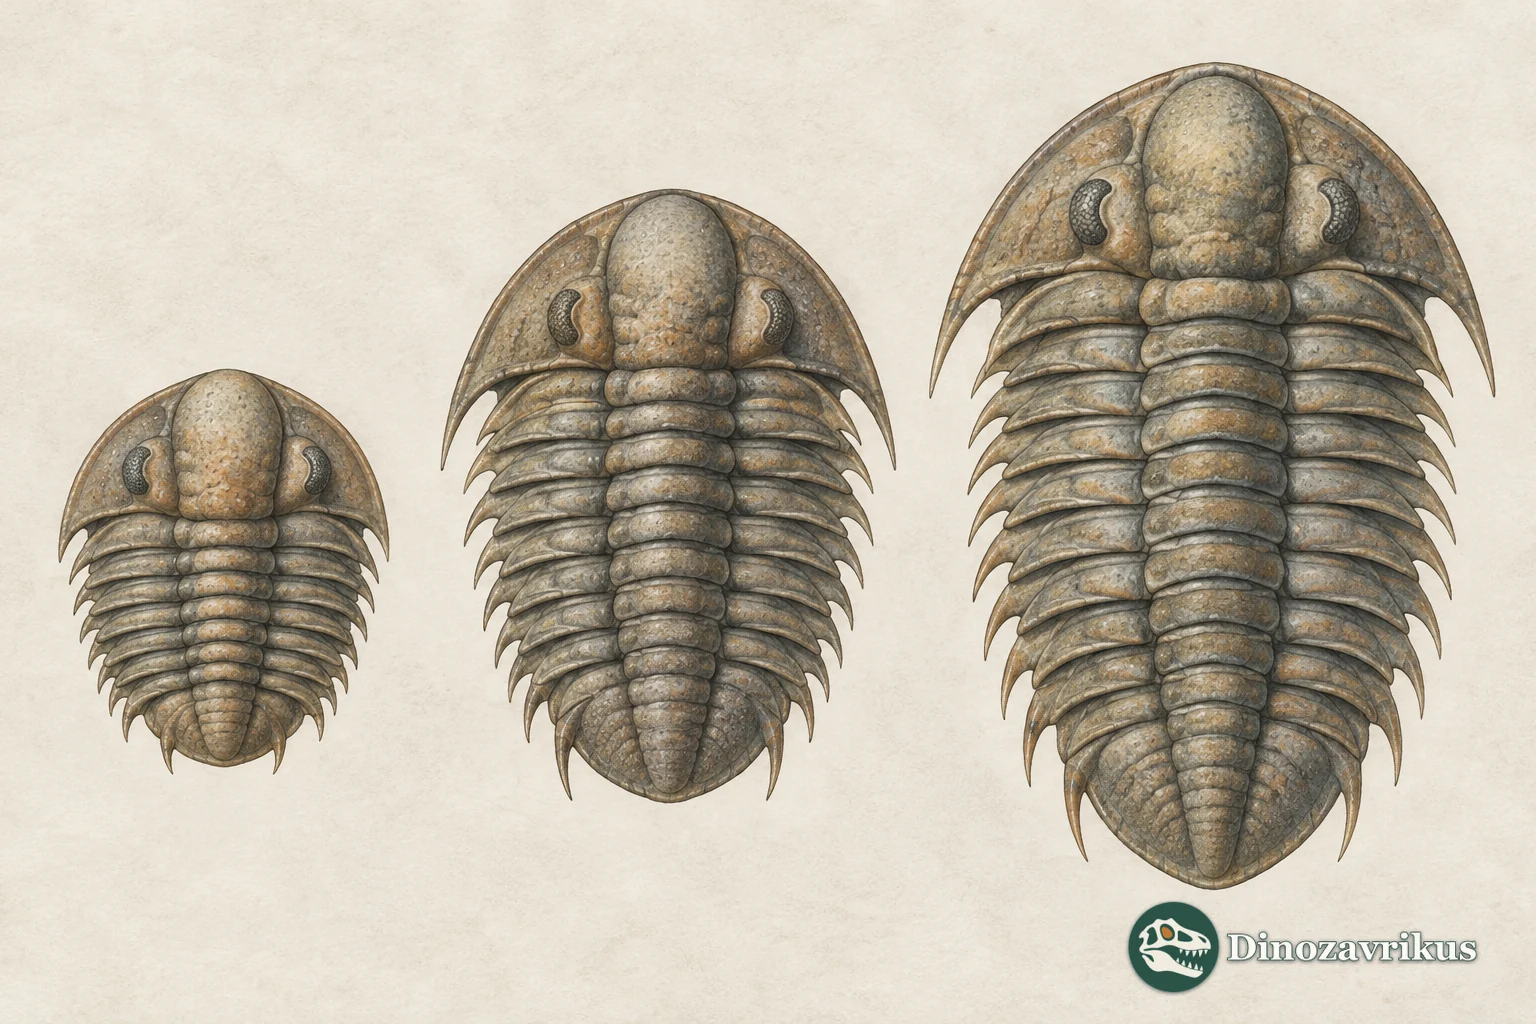
Chatterton, Edgecombe, Vaccari and Waisfeld described growth series of three species from the Argentine Precordillera: T. calandria, T. chingolo and T. problematica. Late in the meraspid phase, their body proportions changed markedly. The authors described the shift as a metamorphosis-like transition, not a pupal stage; trilobites continued through a series of moults.
The same study documented distinctive hypostomes, the plates under the head, with long anterior wings that spread outward and upward. These are observations from particular species and specimens. They do not show that every Telephina had identical larval stages or that a specific habitat change occurred at the same moment.
Food and the limits of reconstruction
No gut contents or direct feeding trace establishes the diet of the genus. A water-column habit could have involved small animals or suspended organic material, but the available shells do not distinguish those possibilities. The visual system of Phacops also invites comparison, yet its anatomy and ecology cannot be transferred directly to Telephina.
Fossils establish the hard shell, eyes, spines and growth stages in named species. Swimming posture, precise depth, soft appendages, colour, diet and social behaviour remain uncertain or artistic. A careful scene can place Telephina in open water while making clear that this is a reconstruction from several clues, not an observed fossil behaviour.
Frequently asked questions
What is the type species of Telephina?
Telephus fractus, described by Barrande in 1852 from the Upper Ordovician of Bohemia, is the type species.
Why do researchers think Telephina lived in open water?
Large eyes, shell proportions, spines and its occurrence in several marine settings support a pelagic or near-pelagic interpretation. Exact depth and swimming behaviour are unknown.
What was unusual about its growth?
Three Argentine species show a marked late meraspid change in body proportions. The pattern should not be assumed for every species in the genus.
What did Telephina eat?
No direct gut or feeding evidence is known. Its precise diet cannot be identified from the shell.