
Kinkelinella is a genus of microscopic marine ostracods known chiefly from mineralised bivalved carapaces. Its valves are striking under magnification: strong longitudinal ribs cross a fine reticulate surface, and some species have a ventral alar expansion. Those features help researchers compare species, but a ribbed outline alone does not establish a genus-level identification.
The best-documented material comes from Jurassic European sections. Studies include isolated valves, closed carapaces, adults and juveniles. The genus belongs in the ancient arthropod catalogue, where its microscopic fossils illustrate how small benthic organisms can contribute to age correlation and environmental research.
Quick facts
| Scientific name | Kinkelinella Martin, 1960 |
|---|---|
| Type species | Kinkelinella tenuicostati Martin, 1960 |
| Group | Ostracoda, Podocopida, Progonocytheridae |
| Best-supported range | Early Toarcian to Bathonian |
| Diagnostic features | Longitudinal ribs, reticulation and a ventral alar expansion in several species |
| Measured example | K. ventrocarinata holotype valve: 0.63 × 0.42 mm |
| Evidence limit | Soft anatomy, diet and behaviour are rarely preserved |
What can the fossils tell us?
Martin established Kinkelinella in 1960 with K. tenuicostati as its type species. This fixes how the generic name is used; it does not show that every ribbed ostracod valve belongs in the genus.
Descriptions compare outline, ribs, reticulation, hinge and marginal zones. The measured K. ventrocarinata holotype valve is 0.63 mm long and 0.42 mm high. That measurement belongs to one specimen, not to the genus as a whole.
Peniche samples contain multiple size classes and growth stages. Size and ornament can change through moulting, so researchers compare series rather than treating every small valve as a separate species.
K. ventrocarinata is reported from the polymorphum Biozone at Peniche. Its relation to the carbon-isotope excursion is interpreted from sample position and the wider assemblage, not from one valve acting as a clock.
Name, type species and classification
E. Martin established Kinkelinella in 1960 and designated K. tenuicostati as its type species. A type species anchors a genus name when taxonomists revise its boundaries. It is not an average specimen, nor does it justify assigning any similar ribbed valve to the genus.
The genus is placed among podocopid ostracods in Progonocytheridae. Older literature may use different combinations, including species once assigned to Procytheridea. Researchers compare external ornament with the hinge, marginal zones, muscle scars and valve outline. When internal structures are unavailable, an identification is less secure.
Authors have not always treated the boundary with the related genus Ektyphocythere in the same way. Species lists therefore depend on taxonomic scope. A compiled database range can include assignments that have not been reassessed from their original descriptions.
Valves and surface ornament
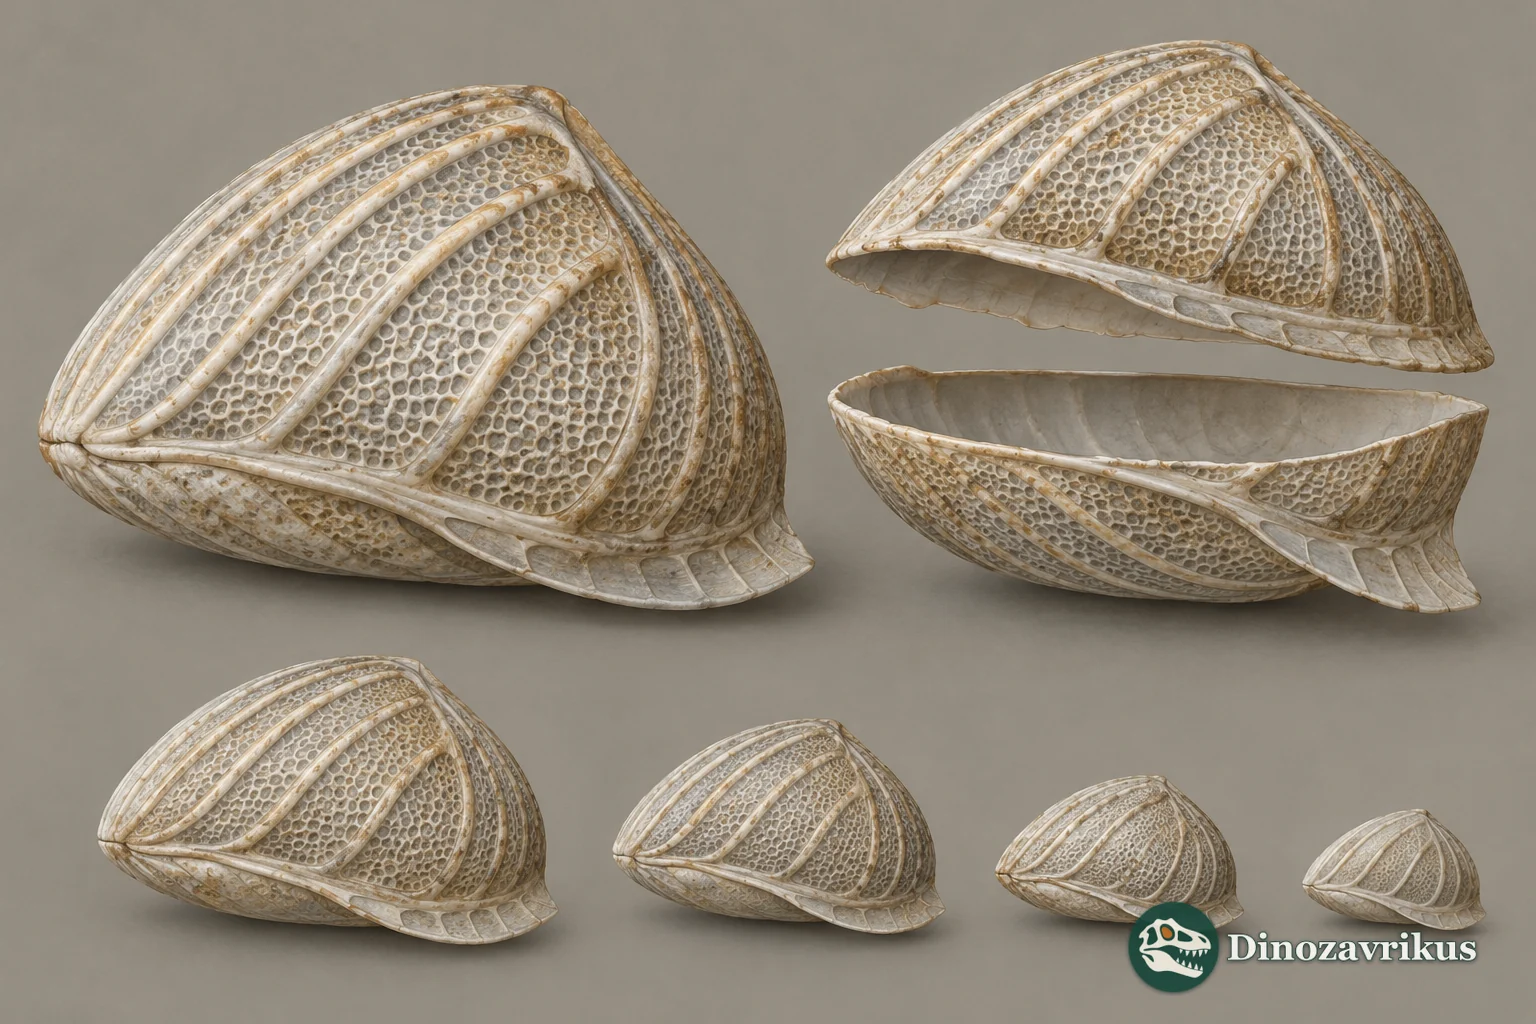
An ostracod carapace consists of two calcitic valves. In lateral view, Kinkelinella valves are often triangular or subrectangular, with a rounded front, a narrower rear and a convex central surface. Several species have a ventral-lateral expansion called an alar wing. It is part of the calcified valve, not a limb or swimming fin.
Longitudinal and oblique ribs cross the surface, with a finer reticulate pattern between them. The number, direction and strength of the ribs vary among species and sometimes among specimens. K. sermoisensis, for example, has been described with strong subvertical ribs and reticulation whose strength varies. Series of valves reveal that range better than a single unusually ornamented fossil.
In Peniche material, K. ventrocarinata has a swollen ornamented carapace and a ventral carina. Its female left-valve holotype, SMF Xe 23886, measures 0.63 mm long and 0.42 mm high. These are specimen-level measurements and should not be treated as a typical size for every species in the genus.
The ribbed relief distinguishes the genus from smoother ostracods such as Acratia and Bairdiacypris. Samarella is another microscopic fossil in the wider arthropod record, but shared scale does not imply the same valve anatomy or close relationship.
Growth, dimorphism and preservation
Ostracods grew by moulting. An animal shed its old carapace and formed a larger one, so a sample may contain several size classes. Juvenile proportions and surface sculpture can differ from adult forms. Researchers examine a growth series before interpreting small size or weaker ornament as evidence for a separate species.
Some ostracod groups show recurring differences between adult carapace shapes that have been linked to sex. Such an interpretation needs repeated patterns, size information and a consistent position in the growth sequence. A single elongated or expanded valve cannot securely identify a male or female. Reproductive soft parts are not known for Kinkelinella.
After death or moulting, the two valves could separate. Currents may sort them by size, while compaction can deform a convex surface. Closed carapaces and isolated valves therefore preserve different taphonomic evidence. Researchers compare articulation, abrasion, orientation, size distribution and surrounding sediment before inferring transport or burial conditions.
Age, localities and biostratigraphy
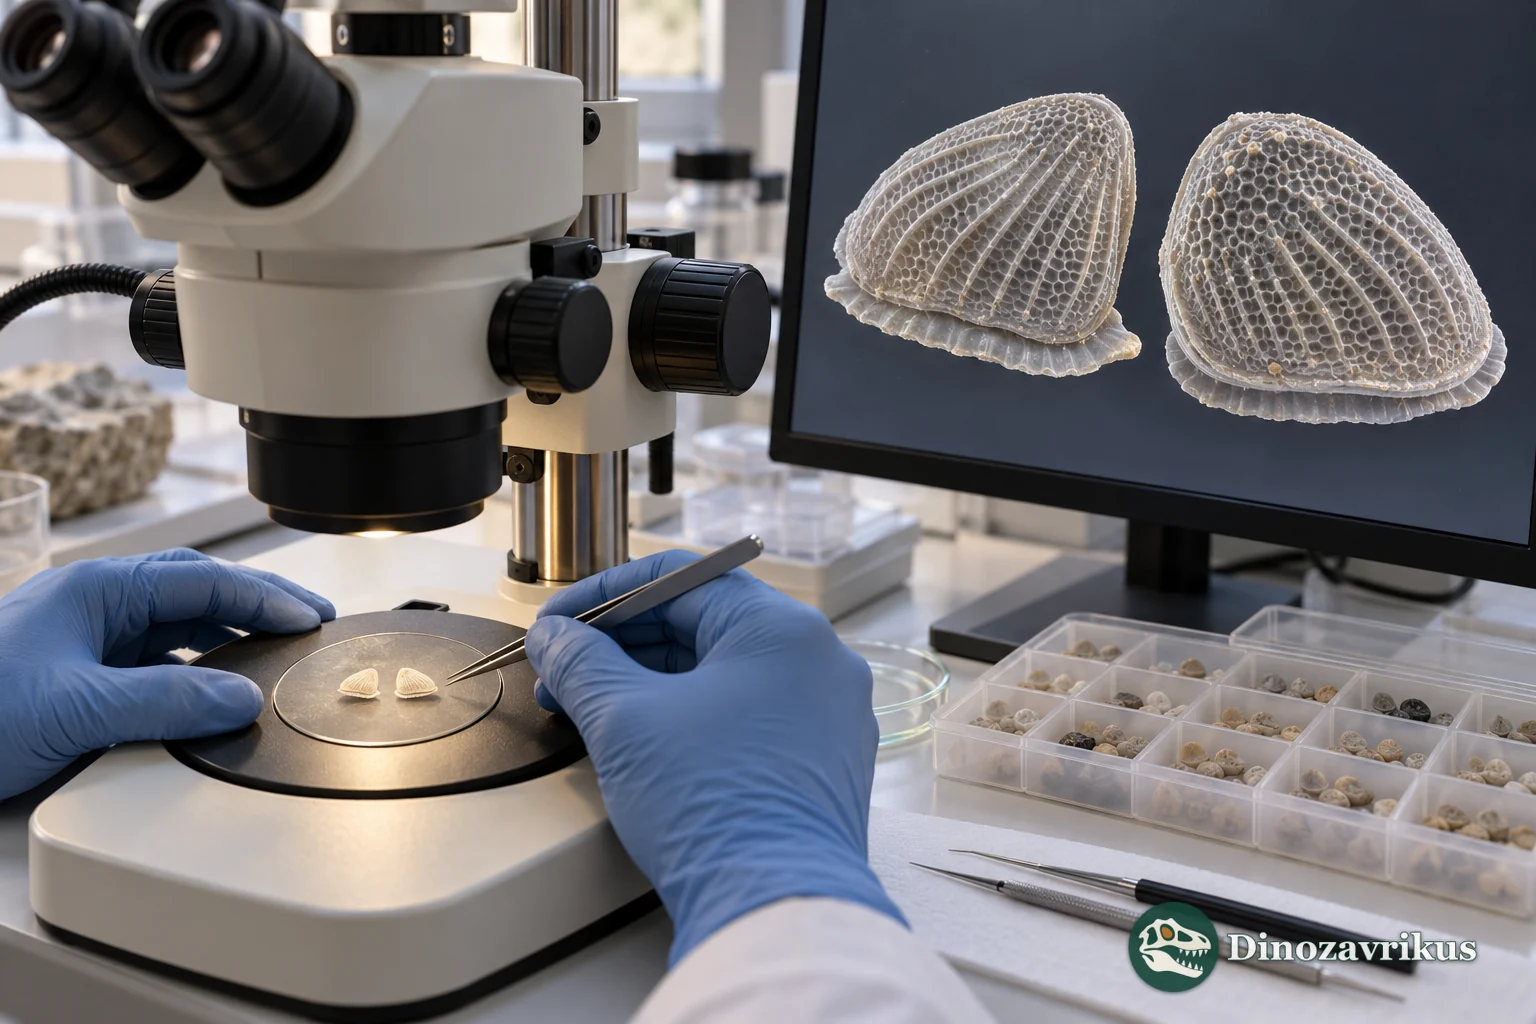
The best-supported published range extends from the earliest Toarcian to the Bathonian. The Toarcian ostracod study of Peniche records the genus from the earliest Toarcian and discusses occurrences into the Bathonian. Earlier database entries, including Triassic assignments, should be checked against their original descriptions before being merged with the well-documented Jurassic record.
Important material comes from Peniche and Rabaçal in Portugal. K. ventrocarinata is reported from the polymorphum Biozone at Rabaçal, where adults and juveniles were collected. Other species have been studied in Toarcian sections in Portugal, Spain and France, and Aalenian–Bajocian faunas in Germany help compare Middle Jurassic communities.
Some ostracod species are useful in zonal stratigraphy when their ranges are short and the identifications are reliable. Kinkelinella is not a geological calendar on its own. At Peniche, the occurrence of K. ventrocarinata is evaluated with the biozone, the rest of the ostracod assemblage and geochemical evidence. That context can place the species near an early Toarcian carbon-isotope event, but one genus is not a direct thermometer or oxygen meter.
Habitat and likely way of life
The genus lived in marine settings, and studied Jurassic assemblages come from marine sedimentary basins. Depth, salinity and oxygen conditions are inferred from the wider rock and fossil assemblage. Ribs on one valve cannot establish whether that animal lived close to shore or farther across a shelf.
Ostracods had limbs and feeding appendages, but those soft parts are rarely preserved with the calcitic carapace. Podocopids could move and collect particles near the bottom, yet the precise diet of Kinkelinella is unknown. There is no direct basis for assigning it filter feeding, predation or a particular behaviour.
When did Kinkelinella live?
The best-documented range begins in the Early Toarcian and continues to the Bathonian. Older compiled records, including Triassic assignments, need taxonomic review.
How large was a Kinkelinella valve?
Ostracods were microscopic. The K. ventrocarinata holotype valve measures 0.63 mm long and 0.42 mm high; those values describe one specimen, not every species.
Was the alar expansion a wing?
No. It is a ventral expansion of the calcified valve, not a limb, fin or flight structure.
Can Kinkelinella date a rock layer by itself?
No. A well-identified species may help correlate a section, but researchers use its stratigraphic position, other fossils and geological evidence together.